
3.1 The light reactions #
3.1.1 Two photosystems, and where they sit #
Leaf anatomy and chloroplast structure belong to Plant Biology and Cell Biology. Palisade mesophyll holds most of the chloroplasts, stomata admit CO2, and veins bring water and remove sucrose. CO2 must still cross the wet wall and the membranes, so mesophyll conductance is a real resistance. Light reactions run in the thylakoid. The Calvin cycle runs in the stroma. PSII is concentrated in the grana. PSI and ATP synthase sit mainly in the stroma lamellae.
Two photosystems work in series because one photon cannot both take electrons from water and reduce NADP+ and still leave a drop for proton pumping. This is the Z-scheme. O2/H2O sits near +0.82 V and NADP+ near −0.32 V. P680+ of PSII, near +1.2 V, oxidises water. The first photon makes a strong reductant, the electron runs downhill to P700+, near +0.5 V, and the second photon at PSI lifts it high enough for ferredoxin. Hill showed that isolated chloroplasts evolve O2 with an artificial acceptor and no CO2 fixation. Ruben and Kamen showed with 18O that the O2 matches the water. Emerson’s red drop is the evidence for two photosystems: far-red light beyond about 680–700 nm drives PSI but not PSII, and shorter-wavelength light restores the yield.
3.1.2 From water to NADP+ #
Antenna complexes, including LHCII, deliver energy to the PSII reaction centre. Charge separation at P680 sends an electron to pheophytin, then QA, then the exchangeable quinone QB. QB, carrying two electrons and two protons from the stroma, leaves as plastoquinol. P680+ is re-reduced by tyrosine Z and then by the oxygen-evolving complex, a Mn4Ca cluster on the lumenal face. The Kok cycle stores four oxidations as S-states. The stoichiometry is 2 H2O → O2 + 4 H+ + 4 e−, with the protons released in the lumen. Four turnovers of each photosystem are required per O2, so linear flow needs at least eight photons per O2. Measured requirements are a little higher.
Plastoquinol is oxidised at cytochrome b6f. Electrons move toward plastocyanin, a lumenal copper protein, and a Q-cycle, the same logic as mitochondrial complex III, deposits extra protons in the lumen. Plastocyanin donates to PSI. P700 passes the electron through chlorophyll, phylloquinone, and iron–sulphur centres to ferredoxin. Ferredoxin–NADP+ reductase makes NADPH. The linear sequence is
H2O → PSII → plastoquinone → cytochrome b6f → plastocyanin → PSI → ferredoxin → NADP+.
The reduced product is NADPH, not NADH. If the plastoquinone pool is over-reduced, a share of LHCII is phosphorylated and moves toward PSI, a state transition that rebalances the antenna.
3.1.3 Cyclic flow and photophosphorylation #
Linear flow makes ATP, NADPH, and O2. Cyclic flow around PSI makes ATP only. Electrons return from ferredoxin to plastoquinone, pass again through cytochrome b6f, and add to the proton gradient without NADPH or O2. In land plants the return requires PGR5 and PGRL1. An NDH complex can do a related job. The chemistry at PGR5 is still argued, so these notes stop at the proteins and the consequence.
The Calvin cycle uses 3 ATP per 2 NADPH. Linear flow’s proton yield falls short of that ratio: spinach chloroplast ATP synthase has 14 c-subunits, so several protons are spent per ATP. Cyclic flow makes up the difference. Photophosphorylation is chemiosmotic. Biochemistry owns the rotary mechanism. Protons accumulate in the lumen and ATP is released in the stroma. In the light the gradient is mostly a ΔpH, which can approach three units, because ion movements dissipate much of the membrane potential. That acid lumen also switches on the protective quenching of Chapter 7.
3.2 The Calvin cycle and photorespiration #
The study of The Calvin cycle and photorespiration provides fundamental principles governing cellular architecture, molecular interactions, and physiological regulation.

Calvin Cycle 5
3.2.1 Rubisco and the cost per CO2 #
Calvin, Benson, and Bassham ordered the cycle with 14CO2. The first stable product is 3-phosphoglycerate. Rubisco adds CO2 and water to ribulose-1,5-bisphosphate and releases two molecules of 3-phosphoglycerate. The same site uses O2 and releases one 3-phosphoglycerate and one 2-phosphoglycolate, because the enediol that CO2 attacks can also be attacked by O2. No Rubisco is known that never oxygenates. The enzyme favours CO2, but air is about 21% O2 and about 0.04% CO2, and the protein is slow, a few turnovers a second. It works only when a lysine is carbamylated and Mg2+ is bound. Rubisco activase spends ATP clearing inhibitory sugar phosphates in the light. In the dark the enzyme quiets, which saves RuBP.
The cycle has three phases. Carboxylation yields two 3-phosphoglycerate per CO2. Reduction phosphorylates each with ATP and reduces each with NADPH, spending 2 ATP and 2 NADPH per CO2. Regeneration rearranges five of every six triose phosphates back to three ribulose-5-phosphate molecules, and phosphoribulokinase spends the third ATP to make RuBP. Net:
| Accounted product | ATP | NADPH |
|---|---|---|
| One CO2 into carbohydrate | 3 | 2 |
| The equivalent of one hexose | 18 | 12 |
Triose phosphate, not free glucose, leaves the chloroplast in exchange for phosphate. Sucrose is made in the cytosol, or starch inside. Thioredoxin, reduced via ferredoxin, switches several regeneration enzymes on in the light. They relax in the dark so the cycle does not run backwards.
3.2.2 Why photorespiration happens, and what it costs #
Photorespiration is the metabolism of 2-phosphoglycolate. It rises when the CO2/O2 ratio at Rubisco falls. Heat lowers specificity for CO2 and lowers the solubility of CO2 faster than that of O2. Drought closes stomata, so intercellular CO2 falls while O2 does not. A hot, dry, sunlit C3 leaf is the case C4 and CAM avoid.
The path crosses three organelles. A chloroplast phosphatase releases glycolate. In the peroxisome, glycolate oxidase makes glyoxylate and hydrogen peroxide, catalase destroys the peroxide, and glycine is formed. In the mitochondrion, two glycines become one serine, one CO2, and one NH3. That is where fixed carbon leaves. The ammonia flux is often greater than primary nitrate assimilation, and GS–GOGAT spends ATP and reduced ferredoxin to recover it. Serine returns through the peroxisome as glycerate, and glycerate kinase spends ATP to remake 3-phosphoglycerate.
Two molecules of 2-phosphoglycolate contain four carbons. One leaves as CO2 and three return, so 75% of that carbon is recovered. This is stoichiometry, not a yield. ATP is spent again, reducing power is lost as peroxide, and net CO2 uptake falls. When CO2 is limiting and light is in excess the path can limit photodamage. It is still a cost.
3.3 Concentrating carbon dioxide #
3.3.1 Kranz anatomy and the Hatch–Slack cycle #
C4 photosynthesis, worked out by Hatch and Slack, concentrates CO2 at Rubisco. Typical anatomy is Kranz anatomy: mesophyll around a thick-walled bundle sheath, joined by plasmodesmata so that C4 acids move and CO2 leaks back slowly. Maize, sugarcane, and sorghum are the examples. A few species manage without Kranz anatomy. It is the usual solution, not a logical necessity.
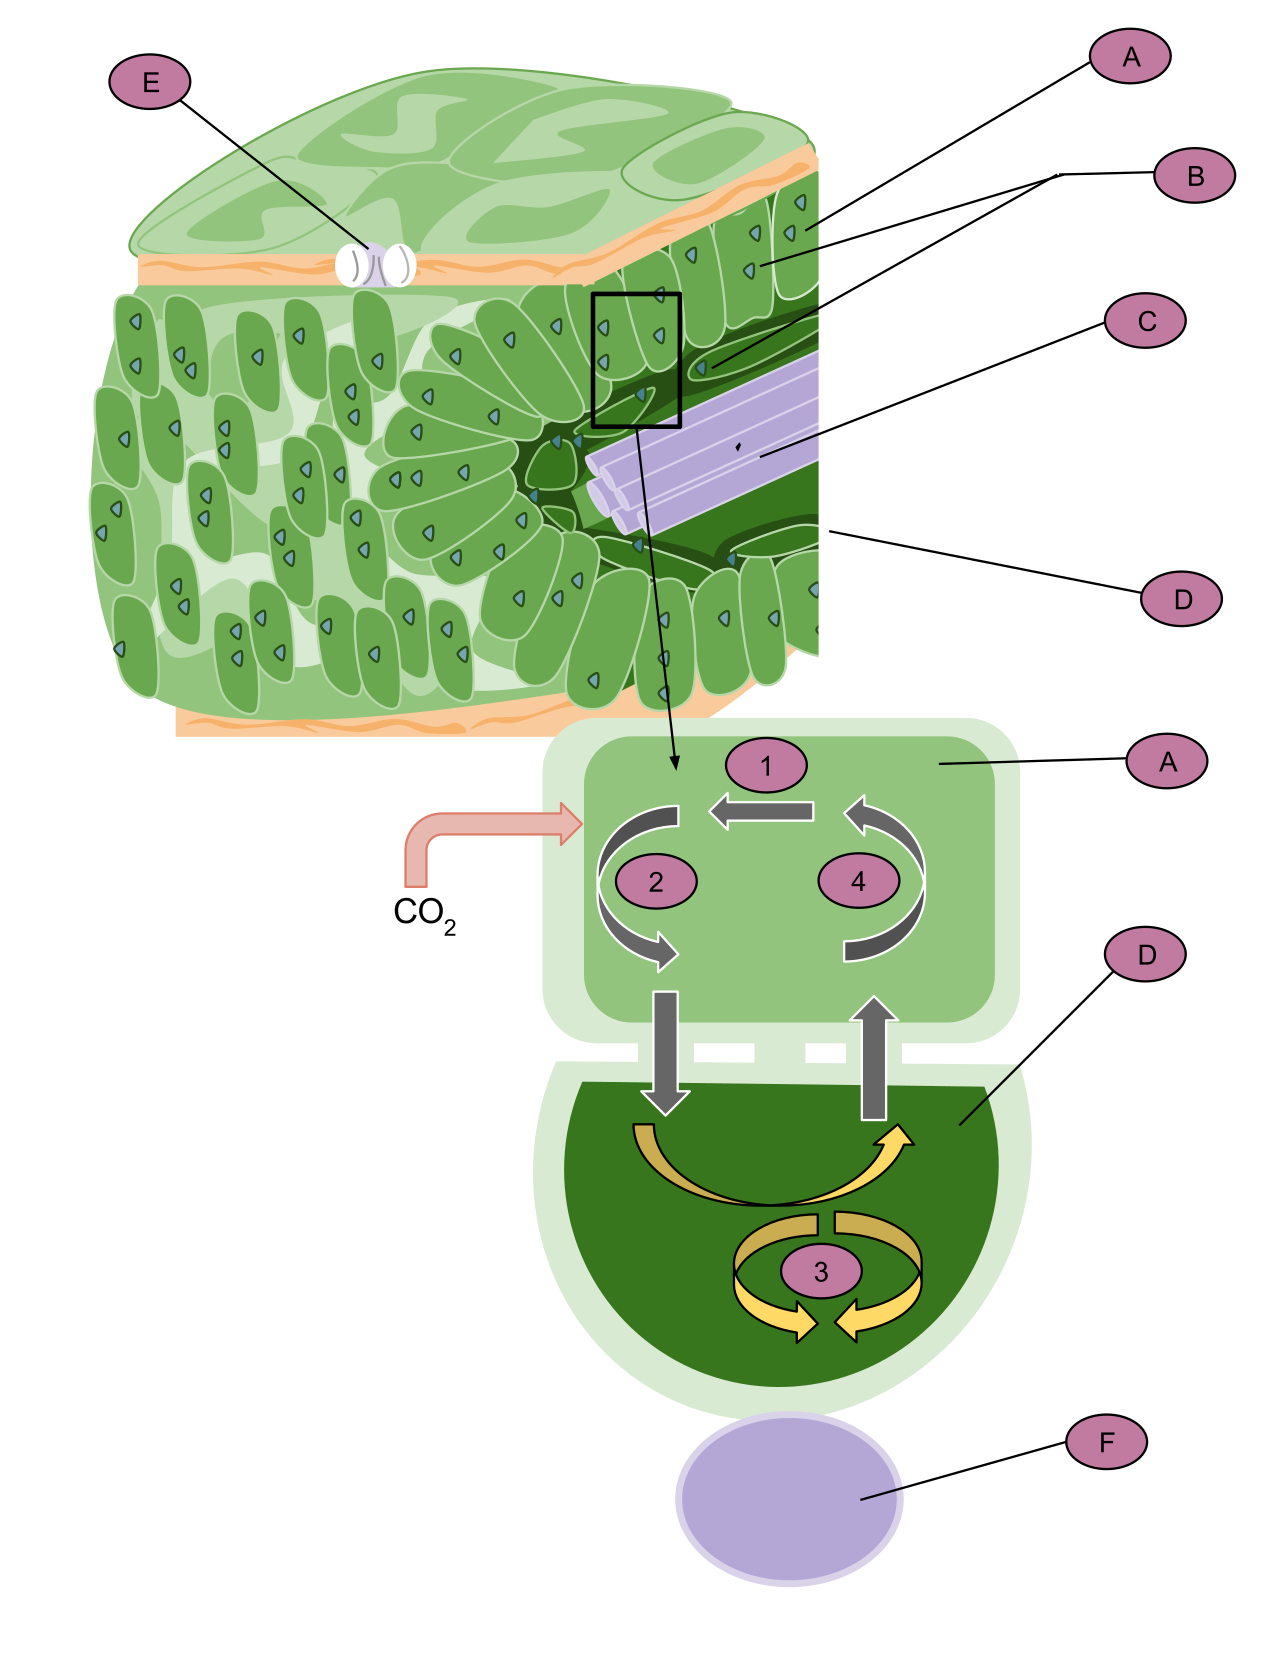
C4 Plant Anatomy
The first carboxylase is PEP carboxylase in the mesophyll cytosol. It uses bicarbonate, does not react with O2, and works at the low CO2 of a partly closed stoma. In maize and sugarcane, the NADP-malic enzyme type, oxaloacetate is reduced to malate, malate moves to the bundle sheath, and decarboxylation releases CO2, pyruvate, and NADPH for Rubisco. Pyruvate returns, and pyruvate phosphate dikinase regenerates PEP at a cost of two ATP equivalents, because ATP becomes AMP. The total is about 5 ATP and 2 NADPH per CO2, against 3 and 2 in C3. Bundle-sheath chloroplasts of this subtype have little PSII, so they evolve little O2 beside Rubisco. NAD-malic enzyme and PEP carboxykinase subtypes decarboxylate a different way. The shuttle is the same idea.
The gains are less photorespiration, a higher temperature optimum, and higher water-use efficiency, because a narrower stoma still feeds PEP carboxylase. Less Rubisco protein can mean less leaf nitrogen. The prices are the extra ATP and cold-sensitive C4 enzymes. C4 is favoured where it is hot, bright, and seasonally dry. Wheat, most trees, and Arabidopsis remain C3.
3.3.2 CAM #
Crassulacean acid metabolism uses the same two carboxylases and separates them in time. Kalanchoë is the classical experimental plant. Cacti and pineapple are the familiar ones. At night the stomata open, when the vapour-pressure difference is smaller. PEP carboxylase makes oxaloacetate, and malate is stored in the vacuole as malic acid, so titratable acidity rises. By day the stomata close, malate is decarboxylated, and Rubisco refixes the CO2 behind closed stomata. Photorespiration stays low because internal CO2 is high.
PEP carboxylase must be off by day or it would recapture the CO2 just released. At night it is phosphorylated and less sensitive to malate. By day it is dephosphorylated and malate inhibits it. The vacuole stores only so much acid in one night, so many CAM plants grow slowly, though pineapple is a real crop. The ice plant shifts from C3 toward CAM under salt or drought. CAM saves water in deserts and in epiphytes. It is not a substitute for C4 in a moist field.
| C3 | C4 | CAM | |
|---|---|---|---|
| First carboxylase | Rubisco | PEP carboxylase, then Rubisco | PEP carboxylase at night, Rubisco by day |
| Separation | None | Spatial, usually Kranz | Temporal |
| Stomata | Open by day | Open by day, often less widely | Open at night |
| Photorespiration | High when hot and bright | Strongly suppressed | Suppressed while daytime stomata are shut |
| ATP per CO2 | 3 | About 5 | C4-acid cost plus Calvin cost, and a storage ceiling |
| Examples | Wheat, rice, most trees | Maize, sugarcane, sorghum | Kalanchoë, cacti, pineapple |
3.3.3 The light-response curve and the CO2 compensation point #
A light-response curve plots net CO2 uptake against photon flux. In the dark the leaf releases CO2. The light compensation point is where photosynthesis equals respiration. The initial slope is the quantum yield, with light limiting. The curve flattens at light saturation, when Rubisco, RuBP regeneration, or triose-phosphate export has taken over. Still brighter light can damage the D1 protein of PSII faster than it is replaced. Full sunlight is about 2000 µmol m−2 s−1. Many C3 leaves saturate at a fraction of that. Maize often does not. A shade leaf saturates sooner than a sun leaf.
C3 quantum yield falls as the leaf warms, because oxygenation takes a larger share of Rubisco. C4 quantum yield is a little lower when photorespiration is slight, because of the extra ATP, and it barely changes with temperature. At high temperature the comparison favours C4.
The CO2 compensation point is the intercellular CO2 at which net exchange is zero. In warm C3 leaves it is typically about 40–50 ppm, and it rises with temperature. In C4 leaves it is close to zero, often only a few ppm, because the pump supplies Rubisco and photorespired CO2 is refixed before it escapes. Present atmospheric CO2 is a little above 400 ppm, far above either point and still not fully saturating for C3 Rubisco in bright light. C4 leaves are already close to CO2 saturation.
3.4 Key terms, summary, and self-check #
Key terms. Z-scheme; oxygen-evolving complex; cytochrome b6f; plastocyanin; ferredoxin; cyclic electron flow; Rubisco; photorespiration; Kranz anatomy; PEP carboxylase; CAM; light compensation point; CO2 compensation point.
Summary. Two photosystems move electrons from water to NADP+ and, with cyclic flow around PSI, supply the 3 ATP and 2 NADPH each CO2 costs. Rubisco also oxygenates RuBP. Photorespiration, through the peroxisome and the mitochondrion, recovers 75% of the carbon in phosphoglycolate and releases CO2 and ammonia. C4 and CAM concentrate CO2 at Rubisco, in space or between night and day, at an extra ATP cost. C3 compensation points lie near 40–50 ppm. C4 compensation points lie near zero.
Self-check.
1. Order the carriers from water to NADP+. Where do the protons that drive ATP synthesis accumulate, and why is cyclic flow still needed?
2. How many ATP and NADPH does one CO2 cost in a C3 leaf, and which phase spends the third ATP?
3. Where in photorespiration are H2O2 and CO2 produced, and what fraction of the carbon in 2-phosphoglycolate returns as 3-phosphoglycerate?
4. What does the extra ATP of the maize C4 cycle buy, and why is the CO2 compensation point of that leaf near zero?
5. On a light-response curve, what is happening at the compensation point, and what replaces light as the limitation once the curve is flat?
