
1.1 Fixity and the idea of change #
1.1.1 Species treated as fixed #
For much of the eighteenth century each species was treated as created in essentially its present form. Linnaeus built a nested classification and, for most of his career, treated species as fixed. Nesting described similarity. Darwin’s reading is that nesting is what a branching genealogy leaves behind.
Buffon and Erasmus Darwin already allowed that species might change. The nineteenth-century break was a mechanism that could be tested, not the first suggestion of change. In these notes the fact is that populations change and that living species share descent. The theories — selection, drift, mutation, migration — are accounts of how. A failed story about one trait does not restore fixity.
1.1.2 Lamarck’s hypothesis #
Jean-Baptiste Lamarck, in Philosophie zoologique (1809), argued that species change. Organs that are used grow; organs that are disused waste; and the acquired change is inherited. Use and disuse was his adaptive mechanism. Inheritance of acquired characters was his hereditary mechanism. The giraffe that stretches, and bears a calf with a longer neck, is the textbook picture of both.
Use does change a body. What fails is the transfer. In animals the germline is set aside from the soma, so a change in muscle or bone is not written into sperm and eggs. Weismann’s tail-cutting is a poor illustration: Lamarck required use, not amputation. There is no general reverse translation from a somatic protein into the germline genome.
Some chromatin marks, small RNAs, and maternal effects do cross a few generations, more readily in plants, which do not sequester a germline as animals do. They are usually short-lived, and they are not a general mechanism that builds enzymes or eyes out of what each generation practised. The fuel of adaptation is genetic variation, sorted by selection and drift. How DNA mutates is Molecular Biology.
1.2 Darwin and Wallace #
1.2.1 The argument #
Charles Darwin and Alfred Russel Wallace reached the same core independently. Darwin had been developing it since the late 1830s, after the Beagle (1831–1836). Wallace sent an essay from the Malay archipelago in 1858; extracts were read together at the Linnean Society that year. On the Origin of Species (1859) is the long argument. Priority is shared.
Three conditions, later stated cleanly by Lewontin, are enough. Individuals vary. The variation is at least partly heritable. Reproductive success differs in association with the trait. The next generation then shifts towards the variants that left more offspring. Darwin also stressed a rate of increase beyond the resources. Excess of births is already inside differential success. No planner is required.
Fitness means that reproductive success, not strength or longevity. A weak animal that leaves more breeding offspring is fitter than a strong one that leaves none. Spencer’s “survival of the fittest” hides this. Artificial selection, which Darwin illustrated with pigeons, shows that heritable variation can be reshaped when only some individuals breed. It is not natural selection: a person supplies the differential. Wallace later disagreed about the human mind and about sexual selection. The shared claim is the three conditions. Sexual selection is Chapter 3.
1.2.2 What Darwin could not yet know #
Darwin had no workable inheritance. Blending — offspring intermediate between the parents — would destroy variation every generation. Mendel, publishing in 1866 and rediscovered about 1900, had shown that factors segregate and can pass unchanged through a heterozygote. A recessive allele can hide and reappear. Mendel’s laws do not, by themselves, change allele frequencies: under Chapter 4’s assumptions, segregation returns the frequencies it received. Selection is what makes one allele increase. The synthesis joins those two facts.
The Galápagos finches are now a measured case of selection. They are not the observation from which Darwin built the theory: he had not sorted the specimens by island. Fossils, biogeography, comparative anatomy, and artificial selection did the early work.
1.3 The modern synthesis #
1.3.1 Mendelism joined to selection #
Between about 1918 and 1950 the objection that Mendelism is discrete while evolution is continuous was answered, and selection was put back at the centre.

Patterns Of Natural Selection
Ronald Fisher showed that many loci of small effect add up to continuous variation and to the correlations among relatives. The Genetical Theory of Natural Selection (1930) made that quantitative. J. B. S. Haldane calculated how fast realistic selection changes allele frequency; the peppered moth was one numerical case. Sewall Wright (1931, 1932) added finite size, drift, inbreeding, and structure. Drift is not in doubt. His “shifting balance” process, in which drift moves a population between peaks of mean fitness, is not established as a common route to adaptation.
Theodosius Dobzhansky’s Genetics and the Origin of Species (1937) took the mathematics back to natural populations. Ernst Mayr’s Systematics and the Origin of Species (1942) added geographic variation and the biological species concept. George Gaylord Simpson’s Tempo and Mode in Evolution (1944) argued that fossil rates fit population genetics. Julian Huxley’s Evolution: The Modern Synthesis (1942) supplied the name. G. Ledyard Stebbins later did the botanical side, including polyploidy.
Orthogenesis — an inner drive along a fixed line — was dropped, as was hopeful-monster saltation as the usual mode. Mutations can have large effects. Ordinary change is still the substitution of many modest differences, fast when selection is strong and very slow when it is not.
1.3.2 Fact and theory #
That populations change, and that living organisms share common ancestry, is as secure as any historical fact in biology. Chapter 2 documents it. Selection is the best-supported cause of adaptive change and has been watched. It is not the only process that changes allele frequencies. Drift, mutation, and migration do too, and much molecular change is not adaptive (Chapter 4).
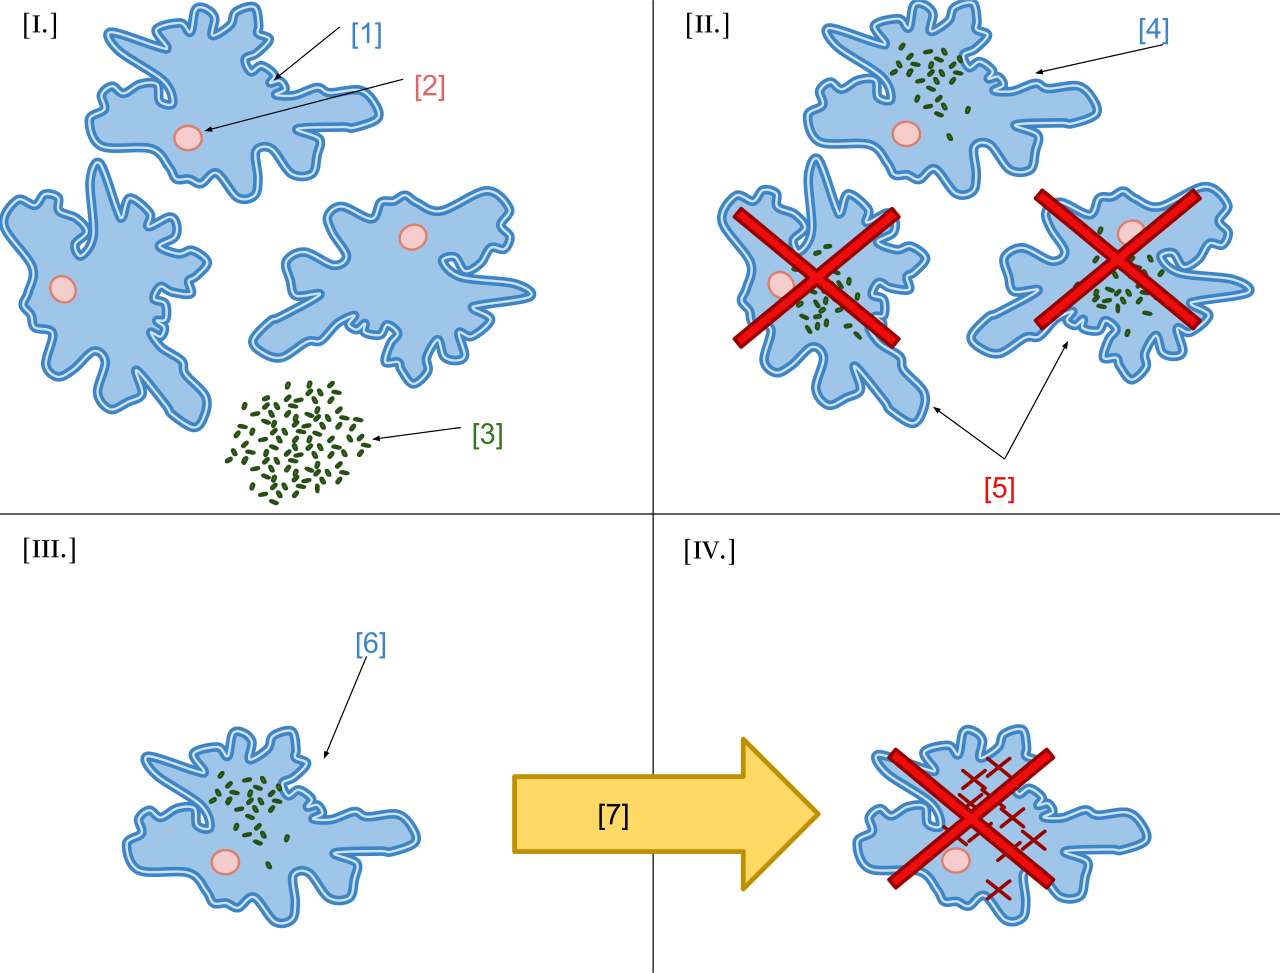
Jeon Experiment- Endosymbiotic Theory Evidence
“Evolution is only a theory” confuses the fact of descent with open questions about which process dominated in a given case: how much of a species difference is selection, and whether a trait was selected for the function now attributed to it. Those questions are real. They are not a list of opinions of equal weight.
1.4 Key terms, summary, and self-check #
Key terms. Fixity; use and disuse; inheritance of acquired characters; germline; heritability; differential reproductive success; artificial selection; particulate inheritance; modern synthesis; orthogenesis.
Summary. Fixity was the default that a nested classification did not by itself overthrow. Lamarck was right that species change and wrong that inheritance of changes acquired by use is the mechanism; short-term epigenetic carry-over is not a substitute. Darwin and Wallace required heritable variation and differential reproductive success. The modern synthesis joined that argument to Mendelian genetics, treated continuous variation as many loci of small effect, and gave drift and geographic speciation a place beside selection. The fact that populations change is not any one theory of how.
Self-check.
1. What, precisely, fails in Lamarck’s account — that use changes a body, or that the change is inherited — and why is tail-cutting a weak illustration?
2. State the three conditions for natural selection without using fitness as a synonym for strength.
3. Why did blending inheritance threaten Darwin, and what fact about Mendelian factors removed the threat?
4. What did Fisher, Wright, and Mayr each add? Which part of Wright’s view remains disputed?
5. Why can selection be rejected for one trait without common ancestry falling with it?
