
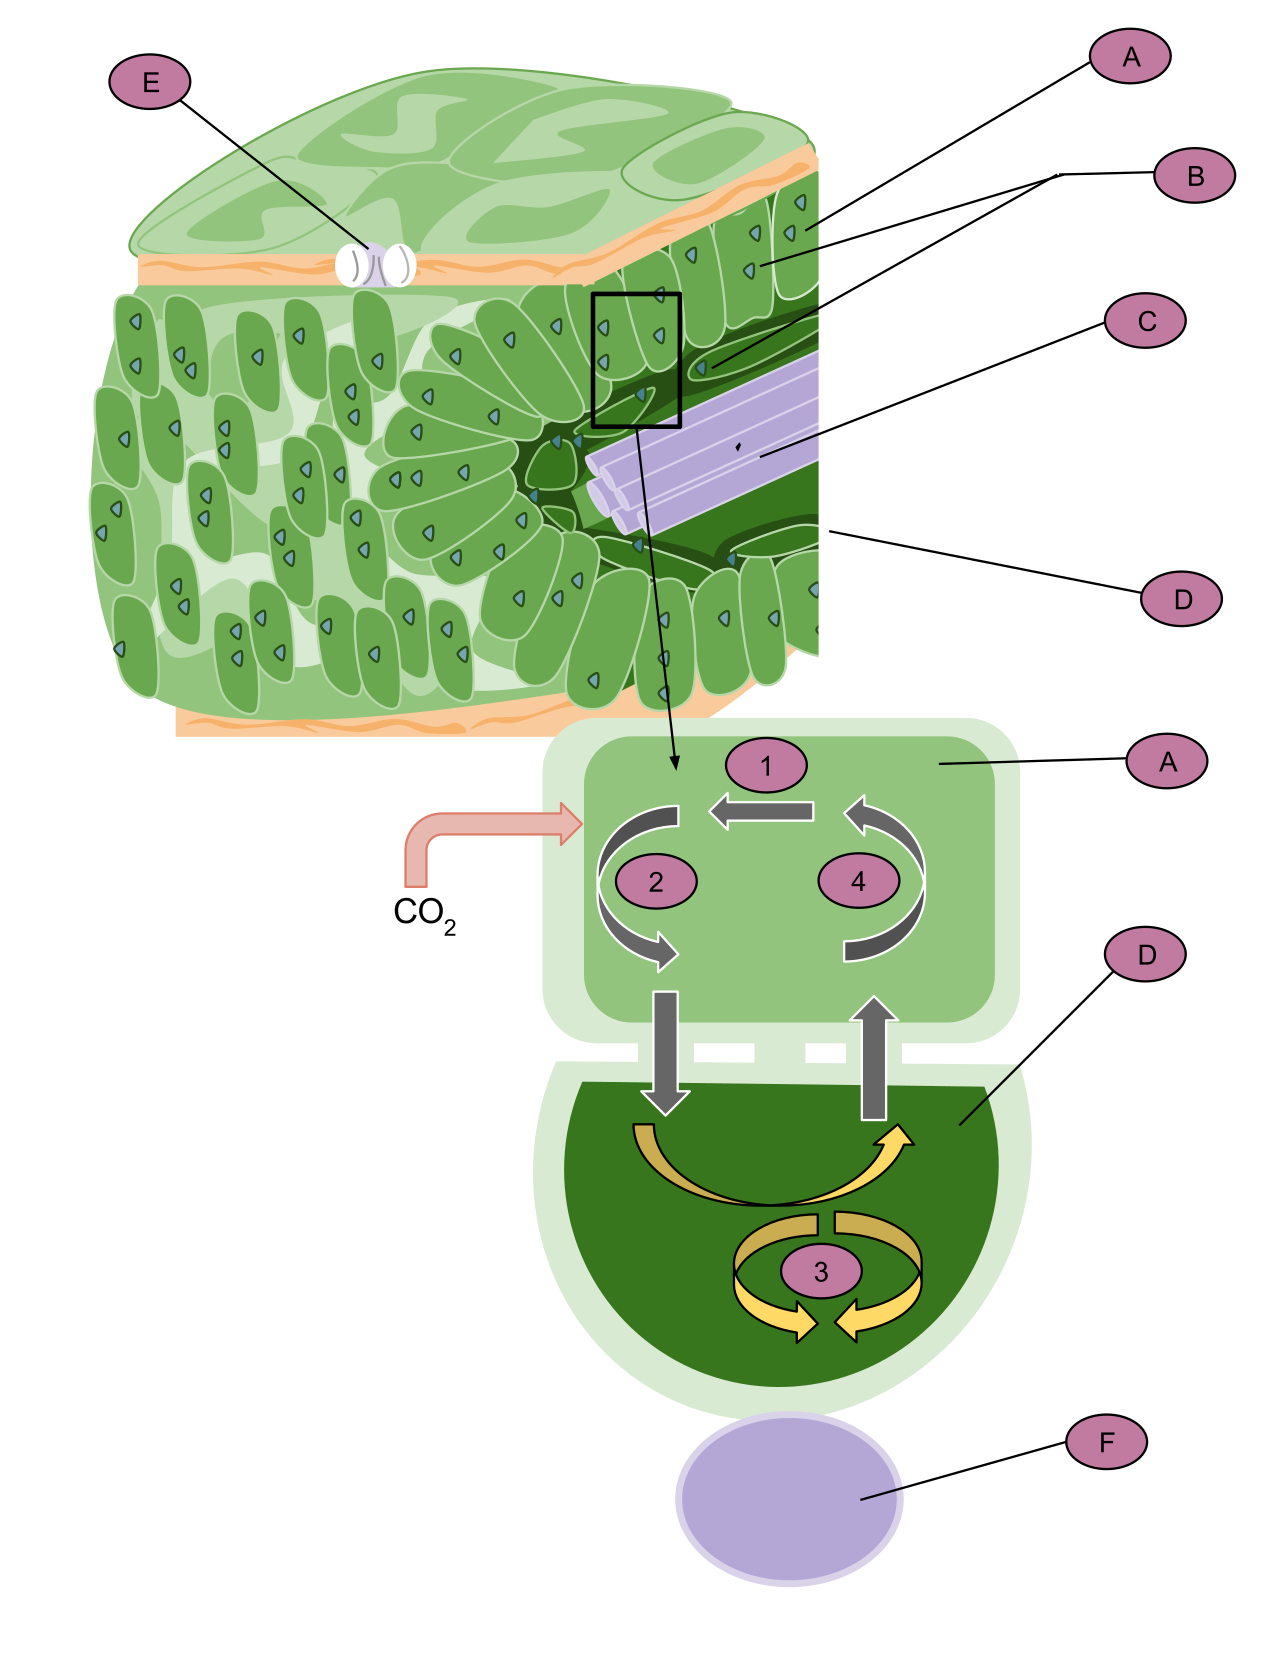
C4 Plant Anatomy
4.1 ATP without a mitochondrion #
4.1.1 Substrate-level phosphorylation and aerobic respiration #
Substrate-level phosphorylation donates a phosphoryl group from an intermediate directly to ADP. Respiration uses a membrane chain to build a proton-motive force, and ATP synthase phosphorylates as protons return. Mitochondria do this on the inner membrane. Bacteria and archaea do it on the plasma membrane.
Glycolysis of glucose to two pyruvates nets two ATP and two NADH. The citric-acid cycle adds one substrate-level ATP or GTP and a load of electrons. Those electrons make more ATP only if the carriers are reoxidised. With oxygen, a modular bacterial chain reduces it to water. The ATP tally is not a fixed integer: textbook proton counts often put a full aerobic balance near thirty per glucose, and the number moves if the chain changes. Fermentation has no such chain. The proton-motive force also turns flagella and drives transport.
4.1.2 Anaerobic respiration and fermentation #
Anaerobic respiration keeps the chain and changes the external acceptor. Denitrifiers such as Pseudomonas and Paracoccus reduce nitrate to N2 through nitrite, NO, and N2O. E. coli reduces nitrate only as far as nitrite. It respires nitrate; it is not a denitrifier. Sulfate reducers such as Desulfovibrio make sulfide, at a still smaller yield, because the acceptor potential is closer to the donor. Assimilatory nitrate reduction builds ammonia for biosynthesis and costs energy. Only dissimilatory reduction is respiration. Methanogenesis — CO2 plus H2, or acetate, to methane — is a separate archaeal energy metabolism. Some cells respire ferric iron. The rule is the same: external acceptor, chain, lower yield than oxygen.
Fermentation regenerates NAD+ on an organic product of the substrate. ATP is only the substrate-level pair, two per glucose in the glycolytic cases. Homolactic organisms (Lactococcus, many lactobacilli and streptococci) make essentially only lactate. Heterolactic Leuconostoc also releases ethanol and CO2. Yeast makes ethanol and the CO2 that leavens bread; Zymomonas reaches ethanol by the Entner–Doudoroff path. Mixed-acid fermentation in E. coli yields lactate, acetate, succinate, formate, and ethanol, and formate is often split to H2 and CO2. Enterobacter makes 2,3-butanediol and less acid. Acetic-acid bacteria oxidise ethanol with oxygen. That is not a fermentation, which is why vinegar is not wine spoilt in the same way (Chapter 9).
4.2 Light and nitrogen #
4.2.1 Oxygenic and anoxygenic photosynthesis #
Light, in organisms that fix CO2, supplies ATP and reducing power. The chloroplast is cell biology. The Calvin cycle is biochemistry. The microbial contrast is cyanobacteria against purple sulfur bacteria. Chloroplasts are the cyanobacterial machine inside a eukaryote.
| Cyanobacteria | Purple sulfur bacteria | |
|---|---|---|
| Photosystems | two, in series | one |
| Pigment | chlorophyll a | bacteriochlorophyll |
| Donor | water | H2S or other reduced sulfur |
| Released | oxygen | no oxygen; sulfur is deposited |
| Habitat | oxic and lit | anoxic, still lit, sulfide present |
| Carbon | Calvin cycle | Calvin cycle in the classical species |
Pulling electrons from water needs a stronger oxidant than pulling them from sulfide, hence a second photosystem. The cost to neighbours is oxygen. Purple sulfur bacteria sit where light meets sulfide and deposit sulfur. Many green sulfur bacteria fix CO2 by a reverse citric-acid cycle, so the Calvin cycle is not the definition of autotrophy. Purple non-sulfur bacteria usually photoheterotroph on organic acids. Bacteriorhodopsin makes a gradient and does not supply a photosynthetic donor.
4.2.2 Nitrogen fixation and the nodule #
The stoichiometry taught for molybdenum nitrogenase is
N2 + 8 H+ + 8 e− + 16 ATP → 2 NH3 + H2 + 16 ADP + 16 Pi.
The iron protein delivers electrons and splits ATP. The molybdenum–iron protein binds N2. Vanadium and iron-only variants exist and are less efficient. Oxygen destroys the enzyme. Clostridium pasteurianum fixes only anaerobically. Azotobacter respires fast enough to keep internal oxygen low and can protect the enzyme reversibly. Anabaena and relatives make heterocysts, thick-walled cells at intervals along the filament, which shut off the oxygenic photosystem, keep nitrogenase, and trade ammonia for carbon with their neighbours. Some cyanobacteria instead fix in the dark.
Rhizobia answer flavonoids with Nod factors, lipochitooligosaccharides. A root hair curls, an infection thread carries the bacteria in, and the cortex builds a nodule. Bacteroids inside a plant membrane still need some oxygen for ATP. Plant leghaemoglobin holds free oxygen very low. The plant assimilates the ammonia; the bacterium receives carbon. Specificity is real: one rhizobium does not nodulate every legume. Nodule development beyond this outline is plant physiology. Heterocysts and leghaemoglobin are two solutions to one constraint.
4.3 Key terms, summary, and self-check #
Key terms. Substrate-level phosphorylation; proton-motive force; denitrification; fermentation; homolactic; mixed-acid; bacteriochlorophyll; nitrogenase; heterocyst; Nod factor; leghaemoglobin; bacteroid.
Summary. Without mitochondria, ATP comes from substrate-level phosphorylation or from a plasma-membrane chain. Nitrate and sulfate replace oxygen at a lower yield; E. coli stops at nitrite. Fermentation regenerates NAD+ on lactate, ethanol, or the mixed-acid set, and nets two ATP per glucose in the first two. Cyanobacteria split water with two photosystems. Purple sulfur bacteria use sulfide, bacteriochlorophyll, and one photosystem. Nitrogenase costs at least sixteen ATP per N2 and cannot meet oxygen; heterocysts and leghaemoglobin each keep the meeting from happening.
Self-check.
1. Where is the E. coli respiratory chain, and what must fermentation regenerate if the chain is off?
2. Why is the sulfate yield lower than the oxygen yield, and why is E. coli not a denitrifier?
3. Name the main products, and one organism, for homolactic, ethanolic, and mixed-acid fermentation.
4. Which two differences between cyanobacteria and purple sulfur bacteria follow directly from the electron donor?
5. Why must a heterocyst lack photosystem II, and what does leghaemoglobin do instead?
