1.1 The Streptophyte Radiation and the Terrestrial Frontier #
The colonization of subaerial land by photosynthetic eukaryotes during the mid-Ordovician (~475–470 million years ago, Ma) stands as one of the most consequential macroevolutionary events in Earth’s biosphere. Terrestrialization altered planetary geochemical cycles, triggered drawdowns of atmospheric carbon dioxide (CO2), accelerated silicate weathering, established modern terrestrial soil horizons (pedogenesis), and provided the bioenergetic substrate for all subsequent terrestrial food webs.
Molecular phylogenomics, nuclear multi-gene coalescent analyses, and plastid phylogenetics decisively demonstrate that land plants (Embryophyta) did not evolve from marine chlorophyte green algae (such as Ulva or Chlamydomonas), but rather from freshwater, desiccation-tolerant charophycean green algae within the lineage Streptophyta. Specifically, sister-group analyses identify the Zygnematophyceae (conjugating green algae) or a clade comprising Zygnematophyceae + Coleochaetales + Charales as the immediate algal sister lineage to embryophytes.
Alternation Of Generations
1.1.1 Ultrastructural and Biochemical Synapomorphies #
Embryophytes share an extraordinary suite of complex biochemical, genetic, and cytological features with advanced streptophyte algae:
1. Rosette Cellulose Synthase Complexes (CSCs): In contrast to the linear CSC terminal complexes found in chlorophytes, streptophytes and embryophytes possess hexameric ‘rosette’ terminal cellulose synthase complexes embedded in the plasma membrane (encoded by CesA multigene families). Each rosette synthesizes an 18-to-36-chain crystalline cellulose microfibril providing high tensile strength.
2. Phragmoplast-Mediated Cytokinesis: During cell division, post-mitotic daughter nuclei are separated by a perpendicular microtubule and actin cytoskeleton array (the phragmoplast). Golgi-derived vesicles travel along microtubules to the division plane, fusing to form a cell plate and establishing primary intercellular cytoplasmic bridges known as plasmodesmata.
3. Peroxisomal Glycolate Oxidase: In photorespiration, phosphoglycolate is metabolized through peroxisomal glycolate oxidase rather than mitochondrial glycolate dehydrogenase (as found in chlorophytes), dramatically increasing carbon salvage efficiency in high-oxygen, high-light terrestrial settings.
4. Flagellar Architecture and Asymmetry: Sperm cells of basal land plants and charalean algae exhibit asymmetric insertion of two subapical whiplash flagella anchored by a multilayered structure (MLS) composed of a microtubular spline and an electron-dense plaque.
5. Polyphenol Biosynthesis & Flavonoid Pathways: Early streptophytes evolved phenylalanine ammonia-lyase (PAL), the gatekeeper enzyme of the phenylpropanoid pathway that converts phenylalanine into cinnamic acid, yielding UV-B protective flavonoids and wall-strengthening polyphenolics.
| Trait / Feature | Chlorophyte Algae (e.g., Chlamydomonas, Volvox) | Streptophyte Algae (e.g., Chara, Spirogyra) | Terrestrial Embryophytes (Land Plants) |
|---|---|---|---|
| Cytokinesis Mechanism | Phycoplast (microtubules parallel to cell plate) | Phragmoplast (microtubules perpendicular to plate) | Phragmoplast with plasmodesmatal connectivity |
| Cellulose Synthase Array | Linear terminal complexes | Hexameric Rosette complexes (hexamers of CesA) | Hexameric Rosette complexes (CesA gene superfamily) |
| Photorespiratory Enzyme | Glycolate dehydrogenase (mitochondrial) | Glycolate oxidase (peroxisomal) | Glycolate oxidase (peroxisomal glycolate pathway) |
| Embryo Retention | Absent; zygote released into open water | Absent; zygote encysts as resistant hypnozygote | Obligate matrotrophy; embryo retained in archegonium |
| Protective Polymers | Algaenan, sporopollenin-like wall coatings | Polyaromatic phenolic compounds | Chemically stable Sporopollenin & Cuticular waxes |

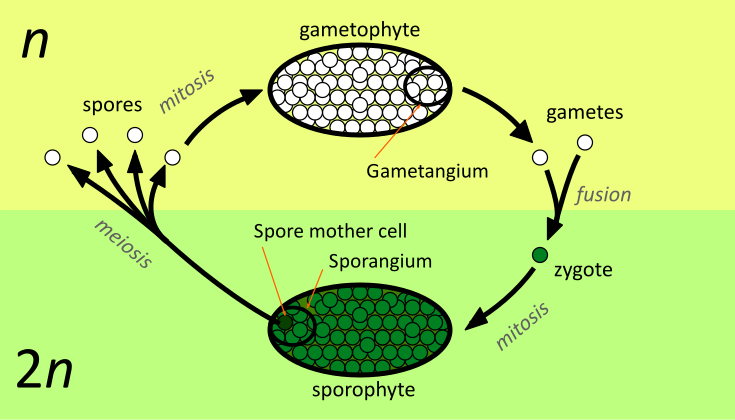
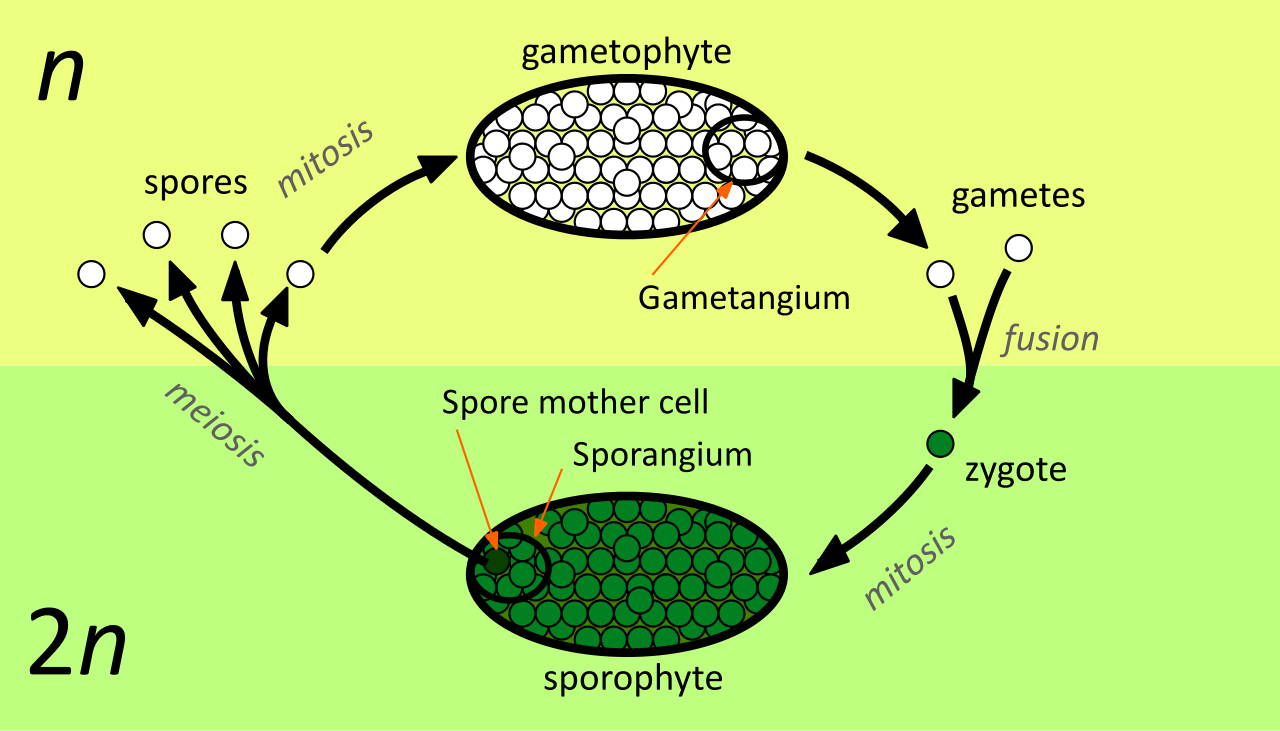
Diplohaplontic
1.2 Overcoming Subaerial Stressors: Cuticle, Stomata & Sporopollenin #
Transition from an aqueous environment where buoyancy, water, and dissolved nutrients were bathed around cells to an aerial regime presented immense physical barriers: desiccation shock, lethal UV-B radiation (280–315 nm), thermal fluctuations, and structural collapse in the absence of hydrostatic buoyancy.
1.2.1 Biogenesis and Architecture of the Plant Cuticle #
The plant cuticle forms an unbroken, hydrophobic outer skin across the aerial epidermis. It consists of two interpenetrating chemical matrices:
- Cutin Matrix: A non-striated, cross-linked polyester biopolymer predominantly composed of hydroxylated and epoxy-substituted C16 and C18 fatty acids (such as 16-hydroxyhexadecanoic acid and 9,10,18-trihydroxyoctadecanoic acid) synthesized by glycerol-3-phosphate acyltransferases (GPATs) and polymerizing cutin synthases (CUS1).
- Cuticular and Epicuticular Waxes: Soluble aliphatic hydrocarbons, long-chain fatty alcohols, free fatty acids (C24–C34), aldehydes, and triterpenoids synthesized in the endoplasmic reticulum via fatty acid elongase (FAE) complexes. These waxes crystalize on the outer cutin surface into microscopic three-dimensional plates, tubes, or films, rendering the boundary non-wettable and reflecting harmful ultraviolet radiation.
1.2.2 Stomatal Architecture and Turgor Dynamics #
While an impermeable waxy cuticle solved desiccation, it choked photosynthetic gas exchange. Land plants resolved this paradox through the innovation of stomata—microscopic epidermal valves formed by a pair of symplastically isolated guard cells flanking a central stomatal pore.
Guard Cells Mechanisms
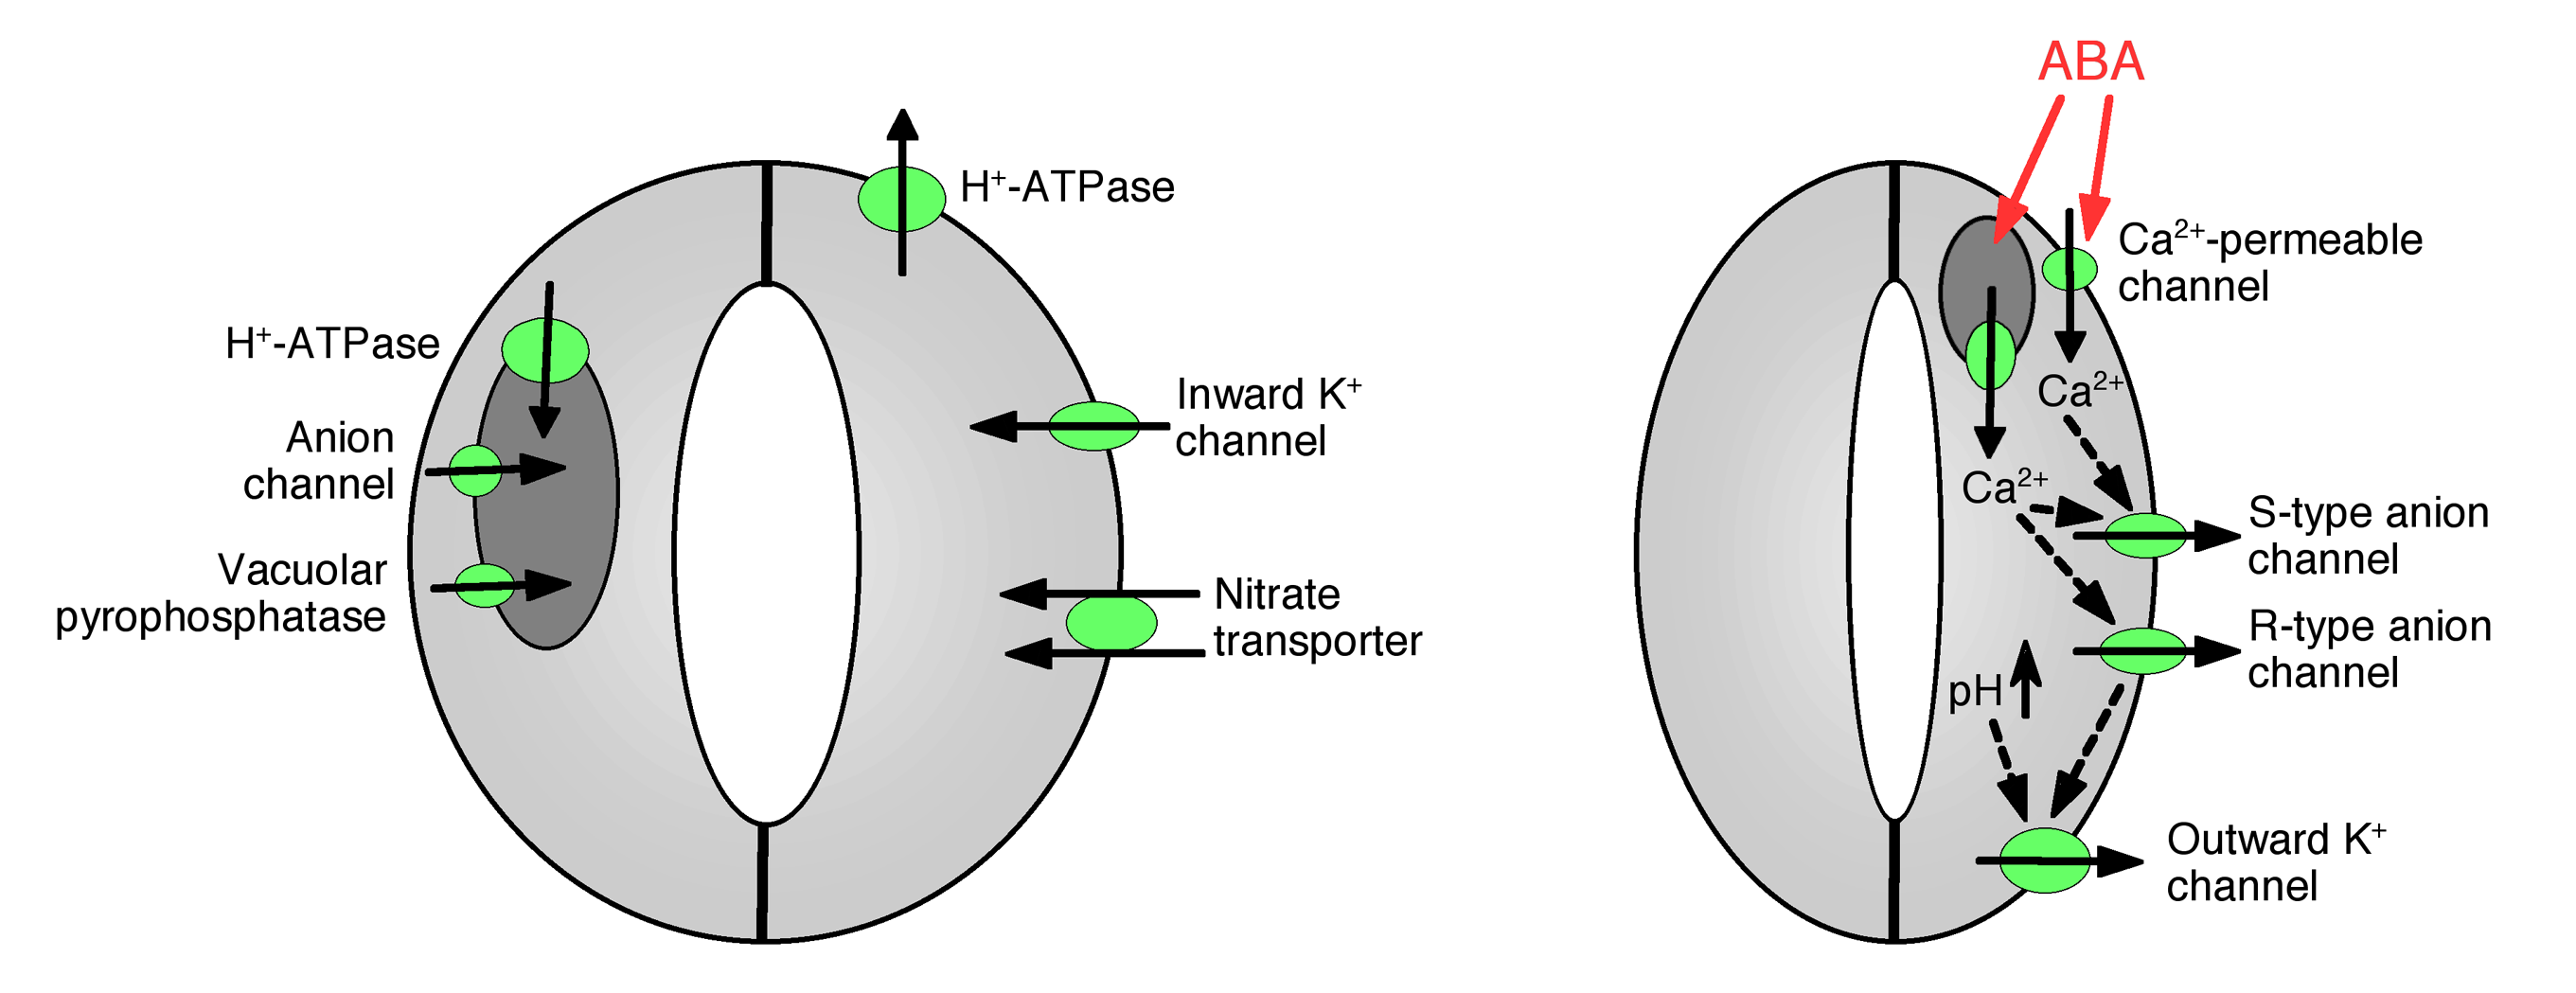
Stomatal movement is governed by osmotic turgor adjustments mediated by electrogenic ion fluxes:
1. Opening Phase (Light / Low Internal CO2): Blue and red light activates plasma membrane H+-ATPases, hyperpolarizing the guard cell membrane to potentials beyond -120 mV. This voltage-gated gradient drives rapid influx of potassium cations (K+) through inward-rectifying channels (KAT1, KAT2) and electrogenic import of chloride anions (Cl–) and organic malate2-. Accumulation of internal solutes depresses osmotic potential (Ψs), driving water influx through aquaporin channels. The differential thickening of guard cell inner walls (cellulose microfibrils oriented radially) causes outward bowing, opening the pore.
2. Closing Phase (Drought / Abscisic Acid [ABA] Signaling): Soil drying triggers synthesis of ABA, which binds to PYR/PYL/RCAR intracellular receptors. This inhibits Type 2C Protein Phosphatases (PP2C), liberating the kinase OST1 (Open Stomata 1). Active OST1 phosphorylates the SLAC1 anion channel, triggering rapid efflux of Cl– and malate, depolarizing the membrane and forcing massive K+ efflux through outward-rectifying GORK channels. The loss of turgor flattens guard cells, sealing the aperture.
1.2.3 Sporopollenin Biochemistry and Spore Wall Architecture #
Dispersal through air required desiccation-resistant propagules. Spores of land plants are coated with sporopollenin, the most resilient biological polymer known in organic chemistry. Formed via the tapetum or spore exine pathway, sporopollenin consists of oxidative co-polymers of polyhydroxylated aliphatic chains, coumaric and ferulic acids, and cross-linked ether-ester phenolics. Sporopollenin resists non-oxidative enzymatic hydrolysis, acetolysis, microbial decay, and UV-B photolysis, preserving spores in the fossil palynological record since the Ordovician Cryptospore horizons.
Porphyrin / Phenylpropanoid Precursors (PAL Pathway)
                    │
                    ▼
     p-Coumaroyl-CoA + Malonyl-CoA
                    │ [Polyketide Synthases & Cytochromes P450]
                    ▼
          Medium & Long-Chain Aliphatics + Phenolic Monomers
                    │ [Oxidative Condensation via ABCG Transporters]
                    ▼
          Cross-linked SPOROPOLLENIN Network (Exine Matrix)
1.3 Key Takeaways & Exam High-Yield Summary #
- Streptophyte Ancestry: Land plants share common ancestry with Charophycean algae (Zygnematophyceae). Synapomorphies include hexameric rosette CSCs, phragmoplast cytokinesis, plasmodesmata, peroxisomal glycolate oxidase, and asymmetric flagellar roots.
- The Cuticle-Stomata Dyad: The cuticle prevents desiccative water loss, while stomata provide dynamically regulated variable gas conductance controlled by K+, Cl–, and ABA signaling.
- Sporopollenin Armor: Protects airborne spores from UV light and microbial enzymology, ensuring reproductive viability across subaerial habitats.
- CSIR-NET / GATE Trap: Spirulina is a cyanobacterium; Chlorella and Ulva are chlorophytes; Chara and Spirogyra are streptophytes. Land plants evolved exclusively from within Streptophyta.
1.4 Review & Self-Assessment Questions #
1. Which structural feature uniquely aligns Zygnematophyceae and Charales with embryophytes, distinguishing them from Chlorophyceae?
- Answer: Hexameric rosette cellulose synthase complexes and phragmoplast-directed cytokinesis with plasmodesmatal intercellular connections.
2. How does ABA induce stomatal closure under water-deficit stress?
- Answer: ABA binds PYR/PYL/RCAR receptors, relieving PP2C inhibition on OST1 kinase. Active OST1 phosphorylates and opens SLAC1 anion channels, depolarizing the guard cell plasma membrane and activating outward GORK K+ channels, triggering osmotic deflation.